*240* The Hidden Cost of Prolonged Cellular Activity
The report further suggests that this effect may help explain why some individuals preserve stronger immune function despite aging…
240 The Hidden Cost of Prolonged Cellular Activity

The report further suggests that this effect may help explain why some individuals preserve stronger immune function despite aging. However, the same study also reportedly observed a substantially increased risk of lymphoma connected to this phenomenon, leading researchers to describe the discovery as both promising and dangerous at the same time.


The publication therefore presents a highly paradoxical interpretation: the same biological process supposedly preserving youthful cellular properties would also increase the probability of severe instability within the immune system itself. In other words, the cells are described as remaining “young” while simultaneously becoming more associated with pathological proliferation. Of if the cells are truly healthier and biologically rejuvenated, why would their long-term stability deteriorate instead of improving?


It becomes less reliable, less stable, and increasingly fragile over time. The cells could follow a similar biological pattern: a temporary increase in activity may create the appearance of improved performance while slowly weakening long-term stability.


Transformations proceed through disengagement: evolution is governed by loss of coupling.

Within this interpretation, the central issue would mainly involve a progressive depletion of the carbohydrates required to maintain healthy cellular function. For a certain period, this intensified activity could be mistaken for a form of rejuvenation, when it may actually reflect accelerated consumption of essential resources.

The more resources it consumes during this intensified phase, the more difficult it becomes afterward to restore a balanced internal condition. The cell nutrients according to its normal capabilities, but those capabilities may no longer be sufficient to recover excessively depleted.


The apparent preservation of cellular “youth” could therefore represent only a transitional state in which the cells remain highly active for a period before progressively losing their true biological stability.

What is presented as prolonged youthfulness may instead correspond to temporarily intensified cellular activity achieved at the cost of progressively reduced stability, reliability, and long-term cellular health.


— — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — —
Beyond Pathogenic Genes: The Adaptive Architecture Hidden Behind Fungal Transformation
One might initially believe that the discovery of the genes dkl and dfl finally explains how certain fungi acquire the ability to infect humans. The publication presents these genes as major controllers of the transition between environmental and pathogenic forms, suggesting that they occupy.
At first sight, the interpretation appears straightforward: disable these genes and the fungus loses its ability to switch form and invade its host. Such a result naturally encourages the idea that the origin of pathogenicity has been identified.
A closer examination, however, reveals a deeper question. Before any gene can control a transformation, the organism must already possess the structural capacity to undergo that transformation. The fungal cell must already contain the cellular machinery, metabolic flexibility, sensing systems, and morphological possibilities required for multiple modes of existence.
The existence of a genetic switch does not explain the existence of the architecture upon which that switch operates. The presence of a control mechanism demonstrates coordination, but not necessarily origin.

Yet the observations are equally compatible with another possibility: these genes may function primarily as absorbers and integrators of environmental constraints. Rather than creating the adaptive response, they may participate in the reception, processing, and redistribution of external information.
In such a framework, the environment becomes the initiating factor, while the genes act as interfaces allowing the organism to reorganise itself according to changing conditions.
The publication focuses on two visible biological states: yeast and mycelium. However, these states may not represent the fundamental reality of the system. What appears more fundamental is the capacity of the fungal organism to remain functional under different environmental constraints.
The visible morphologies are then consequences rather than causes. If additional forms were discovered tomorrow, the underlying principle would remain unchanged.
The organism would still be responding to environmental variation through structural reorganisation. The specific form adopted would simply reflect the conditions encountered.


The experiment demonstrates that these genes are necessary for the observed transition, but it does not automatically demonstrate that they are the ultimate source of the adaptive capability itself. A bridge is necessary for crossing a river, yet the existence of the bridge does not create the existence of the riverbanks. Likewise, a component may be indispensable for expressing a behaviour without being the origin of the biological potential that makes that behaviour possible.
The apparent pathogenic behaviour emerges when a pre-existing adaptive capacity is expressed under particular conditions. What appears to be aggression is often the visible consequence of a deeper process: the ability of living systems to reorganise themselves in response to environmental change.
This suggests that the most fundamental feature is not infection itself, but the adaptive architecture that allows organisms to remain viable across radically different conditions.
The study becomes even more intriguing when discussing the convergent evolution observed across numerous fungal lineages. Different groups appear to have developed remarkably similar adaptive solutions despite their evolutionary separation.
This observation suggests that pathogenicity may not be the primary objective of the underlying mechanisms. Instead, infection could represent one manifestation of a broader adaptive strategy designed to cope with radically different environments. Human tissues would therefore constitute only one among many possible ecological contexts capable of triggering a structural response.

The locally modify the behaviour of particles

The presence of dust directly modifies the physical conditions of interaction. It introduces a large number of contact points at a very small scale, where energy transfer can take place. In the absence of these particles, energy passes through the medium,
but the possibilities for interaction with matter are significantly reduced. Interactions do not disappear, but they are limited by the number of available contact points.

Dust does not create these interactions, nor does it arbitrarily amplify them. It simply makes their actual realization possible by providing the necessary physical conditions.
Its role is not tied to an added function or a regulatory mechanism. It reflects an observable property: the presence of fine structures increases the number of points where energy can interact with matter.
At this stage, understanding shifts.
Dust can no longer be interpreted as useful or harmful depending on context. It appears as an initial evidence — the direct trace of a system in interaction.
It is neither a goal, nor a problem, nor a solution. It is the manifestation that a process is taking place.

Therefore, attempting to eliminate or fix dust without considering what it reveals means acting on a consequence without understanding the structure that produces it. Dust does not need to be corrected. It simply indicates that the system is active.
In this context, a clarification is necessary. The assumption that intervening in a natural system will allow it to restore itself afterward is incorrect. Once the fundamental conditions of interaction are altered, the system cannot return to its original state. Intervention does not correct — it aggravates and transforms the imbalance.

This is precisely what this type of approach reveals. By attempting to fix, control, or locally modify the behaviour of particles, constraints are introduced that are incompatible with how the environment functions. The short-term effect may appear positive, but it is built on a deeper degradation of the system.

This makes a shift in strategy necessary. It is no longer a matter of correcting the system, but of avoiding disruption to its conditions of operation.

Within this framework, an innovative approach emerges, based on a complete reversal of perspective: a system cannot be “repaired” by imposing constraints on it. Instead, supporting biodiversity requires preserving the continuity of interactions.
Of it without fixation, without external control, and without altering the medium itself.
This shift is fundamental: it is no longer about acting to correct, but about acting without altering.
Marked Structural Evidence
At this level, several statements become directly observable.

- Dust is not secondary — it appears simultaneously with interaction.
- Reducing dust does not eliminate the system — it only reduces its visible manifestation.
- Acting on dust means acting on a manifestation, not on the structure.
- The phenomenon itself persists independently of the intervention.
- Dust reveals two types of interactions: internal processes within the system and its connection with the surrounding environment.


The implications of this interpretation extend beyond fungal biology itself. The discovery no longer points primarily toward “genes of infection.”
Rather, it highlights the existence of a pre-existing adaptive architecture capable of absorbing environmental change and reorganising biological activity accordingly. The transition to a pathogenic state becomes a consequence of this adaptability rather than its fundamental purpose.
What appears at first as a story about virulence gradually transforms into a story about the remarkable capacity of living systems to remain functional when confronted with new constraints.

The publication remains highly valuable because it identifies important components.

Yet its deepest significance may lie elsewhere. Rather than revealing the genes that create pathogenicity, it highlights the existence of an adaptive framework already embedded within the organism.
The capacity to survive, reorganise, and remain functional across radically different environments appears to be the true foundation of the phenomenon. Human infection is therefore not necessarily the central story.
It may simply be one visible expression of a much more universal biological principle: living systems persist because they possess architectures capable of absorbing change and transforming constraint into adaptation.
— — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — —
Chicxulub: A Preserved Deep Environment Rather Than an Impact-Created Habitat?
The Chicxulub crater is frequently presented as a unique natural laboratory for studying deep subsurface habitats that may have been generated or sustained by the aftermath of a giant impact.
According to this interpretation, the collision fractured the crust, created hydrothermal circulation systems, and established conditions favorable to microbial life for extended periods. While this perspective highlights the geological consequences of the impact itself, it may overlook a more fundamental observation concerning the nature of deep environments.
Material exchange is limited, external disturbances are greatly reduced, and structural changes occur on much longer timescales. The deeper one descends, the more the environment becomes dominated by preservation rather than renewal.

This distinction is critical because it changes the direction of causality often assumed in discussions of Chicxulub. The impact certainly modified the geological structure of the region, but it did not create the existence of the deep subsurface itself.
The rocks, mineral systems, pressure regimes, and many of the fundamental geological characteristics already existed before the collision occurred. The impact altered an existing structure; it did not generate the entire deep environment from which later observations are derived.
A common tendency is to attribute present-day observations directly to the dramatic event that made the site famous. However, the impact was a transient phenomenon. Its thermal energy gradually dissipated.

The key question therefore becomes not whether the impact generated conditions favorable to life for a period of time, but whether the observed characteristics of the deep environment primarily originate from the impact at all. If a highly stable subsurface environment already existed, then the crater may have acted less as a creator of habitability and more as an exposure mechanism, revealing geological domains that would otherwise remain inaccessible to direct investigation.

Are We Seeing Sources or Simply Visible Effects?
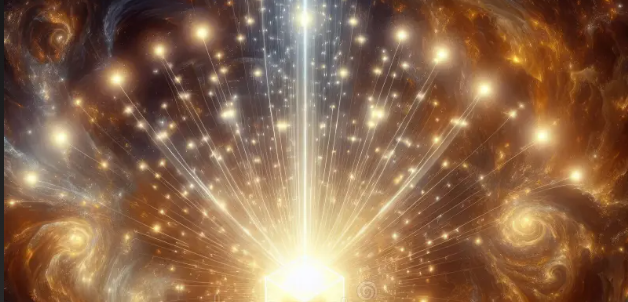
When astronomers observe an image filled with bright points, the usual reaction is simple. Each bright point is considered to be a source. If ten bright points are visible, then ten sources are assumed to exist.
This seems obvious because the light is clearly present in the image.
However, there is a basic question that is rarely asked. Does seeing a bright point automatically prove that it is an independent source?

The observation itself only shows light. It shows a bright central region and many smaller bright points around it. These lights are real because they are observed. But observation and interpretation are not the same thing.
We see many bright spots, yet we know that there is only one lamp. The visible points are real, but they are not independent origins.
The same question can be asked when looking at astronomical images. When a strong central region is surrounded by many bright points, how do we know that every point is an independent source? The image shows the light, but the image does not directly show the origin of each light.

This changes the way the observation can be viewed. Instead of immediately counting sources, we can first ask whether we are looking at sources or manifestations.

In this perspective, the central region becomes particularly important. Rather than treating it as just another object, it may represent the main phenomenon being observed.
The surrounding bright points may then be expressions of that phenomenon rather than completely separate origins.
The key idea is simple. Seeing many bright points does not automatically tell us how many independent sources exist. What we certainly observe are luminous manifestations. The true challenge is determining whether those manifestations come from many separate origins or from a deeper common process.
What I Reveal

The most important distinction is between a source and a manifestation. The image directly shows manifestations. It does not directly show their true origin. Confusing these two ideas can completely change the interpretation.
Opening New Perspectives

Perhaps the first question should not be “How many sources do we see?” but rather “What exactly are we seeing?” Once that distinction is made, the observation becomes richer. The visible points remain real, but their meaning may be very different from what is usually assumed. Sometimes the most important discovery is not found in the light itself, but in the way that light is interpreted.


An important conceptual shift emerges from this perspective. The scientific narrative often emphasizes the processes introduced by the impact: fracturing, heating, fluid circulation, and chemical alteration.
Yet the most persistent feature of the system may not be the disturbance itself but the remarkable stability of the environment beneath it. Deep geological systems are defined by confinement, long-term preservation, and reduced interaction with external processes.
These characteristics exist independently of Chicxulub and would continue to characterize the subsurface even in the absence of the impact event.

The most significant implication is that Chicxulub may owe its scientific value less to its capacity to create a deep habitat and more to its capacity to expose one. The impact was undoubtedly a major geological event, but its effects were temporary when compared with the immense timescales governing deep geological systems.
What remains today is not the impact itself but a subsurface environment whose defining characteristic is stability. In this sense, the crater may be understood not primarily as an engine of habitability, but as a rare geological opening into a largely preserved and comparatively frozen deep world that existed before the collision and continued long after its energy was exhausted.

— — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — — -
메타데이터
- post_id
- d67c798801fd
- slug
- 240-the-hidden-cost-of-prolonged-cellular-activity-d67c798801fd
- url
- https://medium.com/@gouvielos/240-the-hidden-cost-of-prolonged-cellular-activity-d67c798801fd
- canonical_url
- https://medium.com/@gouvielos/240-the-hidden-cost-of-prolonged-cellular-activity-d67c798801fd
- author_url
- https://medium.com/@gouvielos
- status
- ok
- fetched_at
- 2026-10-03 06:18:51